AP Biology · Unit 3 · Topic 3.3
Cellular Energy
A cell must keep building, transporting, repairing, and regulating even when its overall appearance is unchanged. Follow how energy enters a living system, supports work through linked reactions, and eventually disperses to the surroundings. Energy is transformed—not created by enzymes or ATP.
Learning Goals and AP Scope
- Explain why a living system needs a continuing energy supply.
- Reconcile cellular organization with the laws of thermodynamics.
- Describe how ATP connects energy-releasing and energy-requiring processes.
- Predict consequences of blocking a step in a metabolic pathway.
- Use conserved metabolic features as evidence of common ancestry.
The AP focus is conceptual explanation and evidence-based reasoning. The Gibbs free-energy equation is outside the stated AP exam scope. Numerical free-energy examples below are optional extensions, not formulas to memorize for this topic.
1. Energy Transfer Is Different from Matter Cycling
Cells exchange matter and energy with their surroundings. Metabolism includes degradative, or catabolic, pathways and biosynthetic, or anabolic, pathways. These networks transfer energy while rearranging atoms. A carbon atom may pass through many molecules; useful energy must continually be supplied as energy disperses through the system.
Classify the change: a membrane pump establishes an ion gradient, a motor protein moves cargo, and a biosynthetic pathway assembles a molecule. These represent transport, mechanical, and chemical work. They can be linked to a common energy-transfer intermediate even though their products are different.
2. An Ordered Cell Does Not Break Thermodynamic Laws
The first law requires conservation of energy. The second law concerns total entropy: a cell can maintain local organization while its interactions increase the entropy of cell plus surroundings. A growing cell is not an isolated system. Heat transfer and exchanges of matter must be included in the account.
Original energy-budget example: Over a defined interval, a system receives 120 J, exports 75 J as heat, and transfers 25 J as work to its surroundings. If these are all the energy transfers, its stored energy increases by \(120-75-25=20\ \mathrm{J}\). The 75 J has not disappeared; it has left the chosen system.
An organism with roughly constant stored energy can still have substantial energy input and output. A steady state is not the absence of activity, and energy bookkeeping alone is not a calculation of entropy.
3. Follow the Energy; Keep the System Boundary Clear
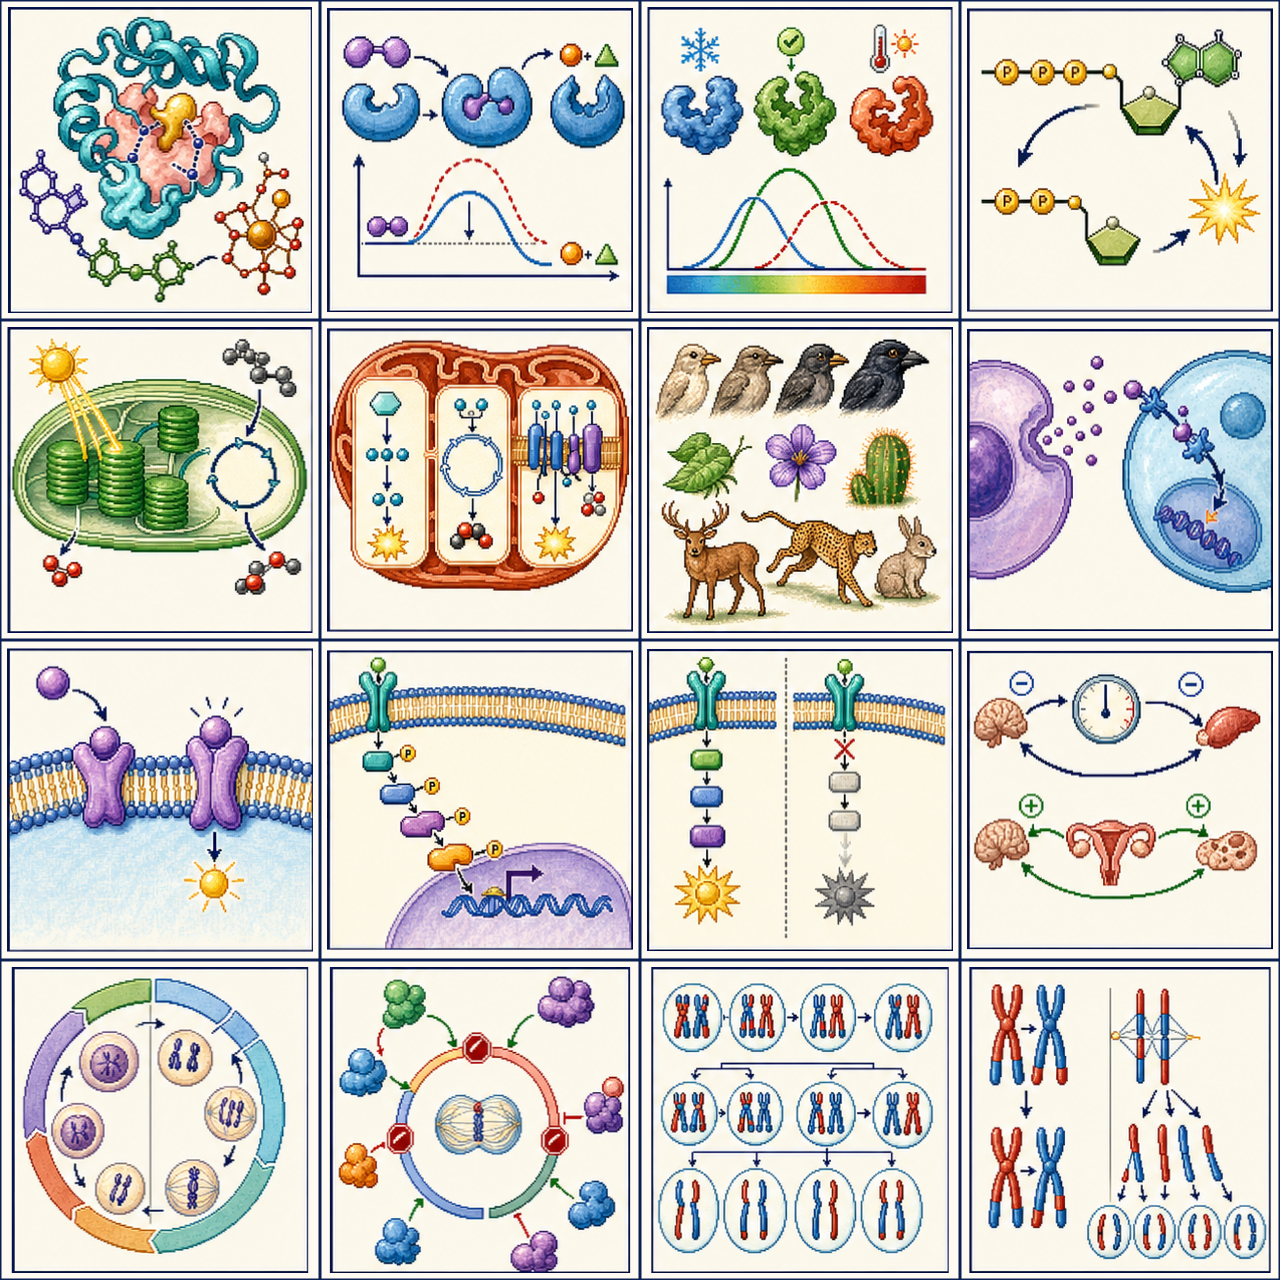
4. Favorability and Speed Answer Different Questions
Free-energy change, written \(\Delta G\), compares products with reactants under specified conditions. A negative value indicates a favorable net forward direction; a positive value indicates that the forward process needs coupling or changed conditions. At equilibrium, the net change is zero. None of these signs alone specifies reaction speed.
Enzymes reduce an activation barrier. They do not change the free-energy difference for the same reaction under the same conditions. “Spontaneous” does not mean instantaneous, and “endergonic” does not mean that an enzyme by itself can supply the required energy.
5. ATP Is a Transfer Intermediate, Not an Energy Source
ATP contains adenine, ribose, and three phosphate groups. Its hydrolysis can be represented in simplified biochemical notation as \(\mathrm{ATP+H_2O\rightarrow ADP+P_i}\), where \(P_i\) denotes inorganic phosphate. Regenerating ATP requires an energy input.
Important correction: breaking a bond requires energy. ATP hydrolysis is favorable because the complete reaction, including formation and stabilization of the products, has a lower final free energy. “High-energy bond” is shorthand for a favorable transfer or hydrolysis reaction, not energy released by bond breaking in isolation.
ATP supports short-term energy transfer. It is not a substitute for longer-term fuel reserves, and recycling ADP does not recycle the energy already dispersed as heat.
6. Coupling Requires a Mechanism
An unfavorable process can proceed when it is physically linked to a sufficiently favorable one. Linkage may involve a shared phosphorylated intermediate or a protein conformation cycle. Hydrolyzing ATP somewhere else in the cell does not automatically drive an unrelated synthesis.
Constructed mechanism model: let X be a molecule with a group that can accept a phosphate. An enzyme first transfers a phosphate from ATP to X, producing X–P and ADP. A second step converts X–P and Y into a combined product XY while releasing phosphate. X–P connects the two steps. This schematic illustrates coupling; it is not a complete chemical equation for a named pathway.
Transport proteins and motor proteins can instead link ATP-dependent state changes to directional transport or movement. The relevant question is always: what connects the energy-releasing event to the work?
7. Optional Extension: Add the Energy Changes
For an invented system under a single specified set of conditions, synthesis requires +18 kJ/mol and its coupled driving reaction contributes −42 kJ/mol per reaction event. With one driving event per synthesis:
What if synthesis instead requires +50 kJ/mol?
One driving event gives \(50-42=+8\ \mathrm{kJ/mol}\), so the specified combined process remains unfavorable. Two driving events would give \(50-84=-34\ \mathrm{kJ/mol}\), but a mechanism must actually couple both events to the synthesis. Arithmetic alone cannot establish that such a mechanism exists.
Real ATP hydrolysis has a condition-dependent free-energy change. Do not treat the invented −42 value as a universal constant or mix values measured under different conditions.
8. Why Metabolism Uses Many Steps
A pathway connects intermediates: \(A\xrightarrow{E_1}B\xrightarrow{E_2}C\xrightarrow{E_3}D\). Individual enzymes control particular transformations. Sequential transfer allows cells to capture energy in usable intermediates and regulate flux rather than releasing all available energy in one uncontrolled event. An overall favorable pathway can still contain energy-requiring steps.
Prediction exercise: If E₂ is inhibited while A continues entering, B may accumulate and C and D may decline. The prediction assumes no effective bypass, no compensating uptake, and continued E₁ activity. If a real dataset disagrees, examine those assumptions rather than discarding the data.
Feedback inhibition can reduce an early step when downstream product is abundant. This regulates production; it does not reverse the laws of thermodynamics.
9. Shared Pathways and Common Ancestry
ATP use and related core energy-transfer machinery occur across the domains of life. Conserved enzyme sequences and reaction organization support inheritance from ancestral systems. Shared function alone is weaker evidence than shared function accompanied by detailed molecular similarities.
Evaluate the claim: “Two organisms both make ATP, so one must be the direct ancestor of the other.” This is not justified. Shared features can support common ancestry without identifying a direct ancestor–descendant relationship. Not every organism retains every pathway, and a shared core can coexist with different enzymes, variants, or losses.
10. Interpret an ATP-Pool Experiment
In a fictional experiment, comparable cell samples begin with the same ATP pool. A treatment reduces ATP regeneration. ATP values are normalized to each sample's initial amount.
| Time (min) | Vehicle control (%) | Treatment (%) |
|---|---|---|
| 0 | 100 | 100 |
| 2 | 99 | 76 |
| 4 | 101 | 53 |
| 6 | 100 | 35 |
Explain the pattern and its limitations
The treated pool falls by 65 percent of its initial amount over six minutes. This is consistent with consumption outpacing regeneration. It does not measure ATP-production rate directly: pool size depends on both production and use. The control's stable pool does not mean that it uses no ATP.
Use independent biological replicates, matched cell numbers, a vehicle control, viability measurements, and a check that the treatment does not interfere with the ATP assay. Additional flux measurements would be needed to separate altered production from altered demand.
11. Connect to Photosynthesis and Respiration
Photosynthetic cells capture light energy; respiratory pathways transfer chemical energy through controlled reactions. Both can use membrane gradients and ATP-generating machinery, but their inputs, electron-transfer routes, and biological roles differ. Plants also respire. Photosynthesis and respiration should not be pictured as the same enzyme pathway running backward.
Reasoning prompt: A membrane becomes leaky to the ions that form its energy-storing gradient. Predict less capacity to drive gradient-dependent work, even if the membrane and its enzymes remain present. The organization of components matters as well as their identities.
12. Check Your Understanding
1. Does building an ordered cell violate the second law?
No. Include the surroundings and energy and matter exchanges. Local organization can be maintained while total entropy increases.
2. Can extra enzyme alone make an unfavorable uncoupled reaction favorable?
No. It can alter rate, not the free-energy difference under fixed conditions. A coupled process or changed conditions are needed.
3. Does a stable ATP concentration prove that ATP is not being used?
No. Regeneration can balance consumption. A pool measurement is not a turnover measurement.
4. What happens if ADP is available but the driving energy supply stops?
ADP availability alone cannot sustain ATP regeneration. Without an alternative energy supply, continued ATP use can deplete the ATP pool and compromise work.
5. A pathway inhibitor lowers the final product. Is the inhibited enzyme necessarily the last one?
No. Blocking an upstream step can limit downstream substrate supply. Measure intermediates and consider bypasses to localize the effect.
Track the energy source, identify the coupling mechanism, and distinguish a stored amount from a flow rate. Connect each claim to a system boundary and evidence.
Concept references: OpenStax Biology 2e, Energy and Metabolism, Free and Activation Energy, Laws of Thermodynamics, and ATP; scope checked against the College Board AP Biology Course and Exam Description, Topic 3.3. Explanations, diagrams, hypothetical mechanisms, numerical data, and worked questions are independently authored for Insomnia Studyroom. Source illustrations and exercises are not reproduced.
Official curriculum reference: College Board AP Biology course page. The explanation and worked example are independently written for this study site.